

Introduction
Restoring degraded forests focuses on recovering and preserving essential ecosystem attributes, such as species diversity, ecological processes, and the complexity of vertical and horizontal structure. This complexity arises from the variety of ages, heights, diameters, number of individuals, and species that make up a community, forest, or ecosystem (Buthia et al., 2019). Forest structural analysis is considered a reliable and repeatable indicator of biodiversity, as well as of the overall health and functioning of the ecosystem in question (Perring et al., 2015). Therefore, the evaluation of structural attributes and monitoring of their changes are essential components of any ecological or forest restoration effort, as they provide valuable information for improving future restoration strategies and for their potential application in ecosystems with different levels of degradation (Lara et al., 2019).
The Society for Ecological Restoration, established in 1988, outlines key attributes that should be considered when determining whether a restored site possesses sufficient biotic and abiotic resources to continue developing without human intervention (Gann et al., 2019; Mola et al., 2018). These attributes include: (1) structure (such as size class distribution, basal area, and density); (2) the presence of native species; (3) functional groups; and (4) reproductive populations of species. Additionally, Mola et al. (2018) emphasize that changes in a restored ecosystem can be evaluated through indicators such as structural complexity, plant and functional diversity, and ecological processes. The attributes assessed in a restored or reforested area must be compared to those of a reference forest, which should be included in any restoration-focused study.
Vegetation structure is considered one of the main attributes evaluated in the context of ecological restoration, as it influences biomass production, biodiversity, and the quality of ecosystem services (Mora-Donjuán et al., 2016; Ni et al., 2014; Rubio-Camacho et al., 2014). Forest stand structure refers to the spatial organization of system components, and it is determined by three primary characteristics: species diversity, species composition, and the spatial distribution of trees (Manzanilla-Quijada et al., 2020; Ni et al., 2014).
Reforestation has been one of the most widely used practices for the recovery of forest ecosystems, offering benefits such as accelerating natural succession processes by modifying the microclimate (Derhé et al., 2016). Due to its significance in restoring deforested and degraded areas, Mexico’s National Forestry Commission (CONAFOR) launched a large-scale forest restoration initiative in 2013 through the implementation of the National Forestry Program (PRONAFOR) for the 2013-2018 period (Méndez-Toribio et al., 2018). However, reforestation represents only the beginning of a long and gradual process of ecosystem recovery. For this reason, the generation of scientific information is also essential to support the understanding and management of ecosystems through restoration and reforestation efforts.
In Mexico, studies on vegetation structure and diversity in reforested areas remain limited. Reforestation efforts are often considered successful based on high survival rates-an important metric, but insufficient to conclude that a reforested site has fully recovered its ecological processes and functions. Therefore, it is essential to directly evaluate attributes such as structural complexity, species diversity, and ecological processes in any reforested area, and to assess the changes that have occurred. Such evaluations help determine whether the site possesses sufficient biotic and abiotic resources to support continued development, whether it can maintain structural and functional integrity, whether it is resilient to future disturbances, and whether it can interact with surrounding ecosystems (Gann et al., 2019; Mola et al., 2018). This study hypothesizes that structural complexity in reforested areas increases with age, gradually approaching that of a reference forest.
The objective of the present study was to compare the vertical and horizontal structure of two Pinus montezumae Lamb. reforested areas of different ages with a reference forest in the northeastern region of the state of Puebla. The aim is to provide information that can support decision-making in programs or initiatives focused on the recovery of degraded areas.
Materials and Methods
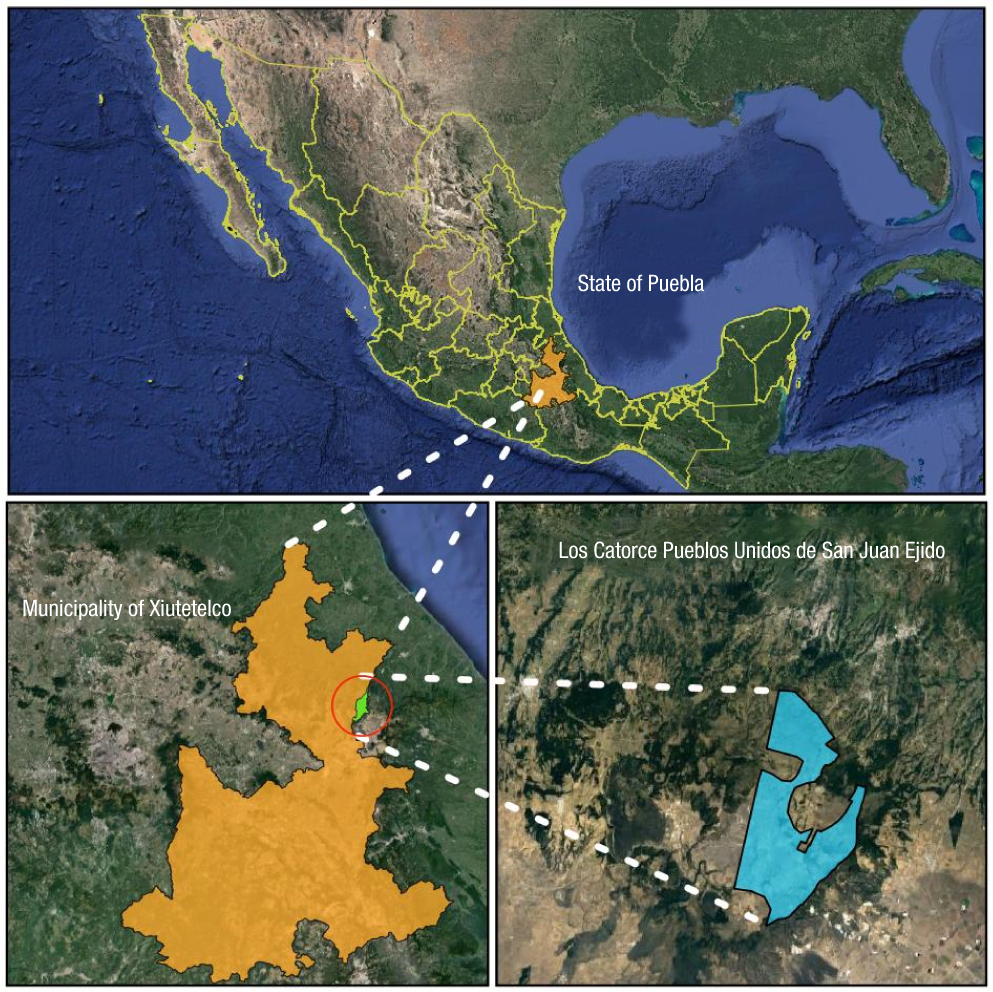
The study was conducted in the Los Catorce Pueblos Unidos de San Juan ejido, located in the municipality of Xiutetelco, in the northeastern region of the state of Puebla. The ejido is located between coordinates 19° 38’ 19.40” N - 97° 24’ 8.71” W and 19° 45’ 12.72” N - 97° 22’ 3.77” W, elevations ranging from 2 500 to 3 000 m (Instituto Nacional de Geografía e Informática [INEGI], 2020) (Figure 1).
The predominant climate in the region is temperate sub-humid, with a mean annual temperature ranging from 12 to 18 °C and an average annual precipitation between 650 and 850 mm (García, 2004). The dominant soil types are Eutric Regosol and Ochric Andosol (INEGI, 2020). The prevailing vegetation consists of coniferous and broadleaf forests composed of Pinus teocote Schiede ex Schltdl. (aztec pine), P. montezumae (Moctezuma pine), P. patula Schiede ex Schltdl. et Cham., and Alnus jorullensis Kunth. (Mexican alder), with transition zones of dry forest that harbor grasses and low-stature tree species typical of semi-arid climates (Comisión Nacional para el Conocimiento y Uso de la Biodiversidad [CONABIO], 2021).
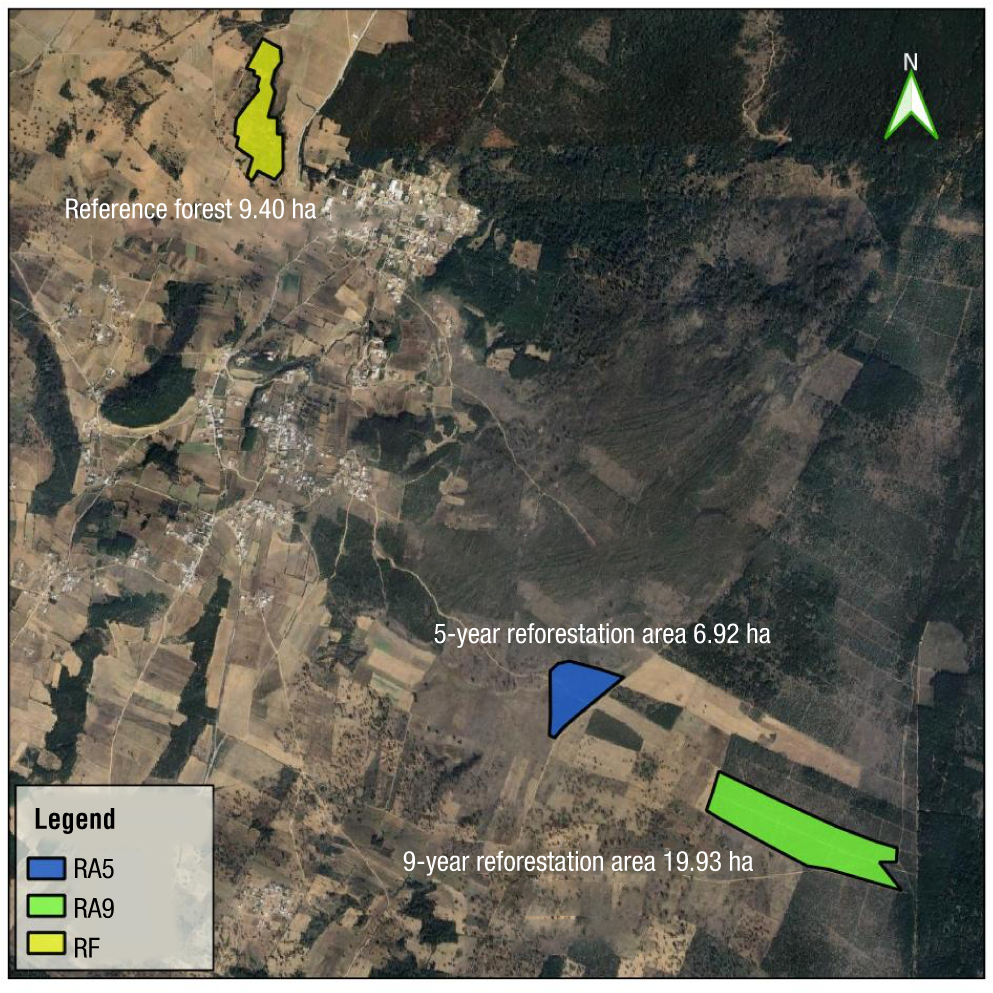
A total of three sites with similar abiotic conditions-aspect, slope, and elevation-were selected near one another: two reforested areas with P. montezumae, planted 5 (RA5) and 9 (RA9) years prior, and a reference forest (RF) composed of P. teocote, P. montezumae, and Alnus jorullensis, with established tree cover (Figure 2). The reference forest is a remnant of the natural forest, with a certain degree of disturbance, serving as a model for planning and evaluating restoration or reforestation efforts (Gann et al., 2019).
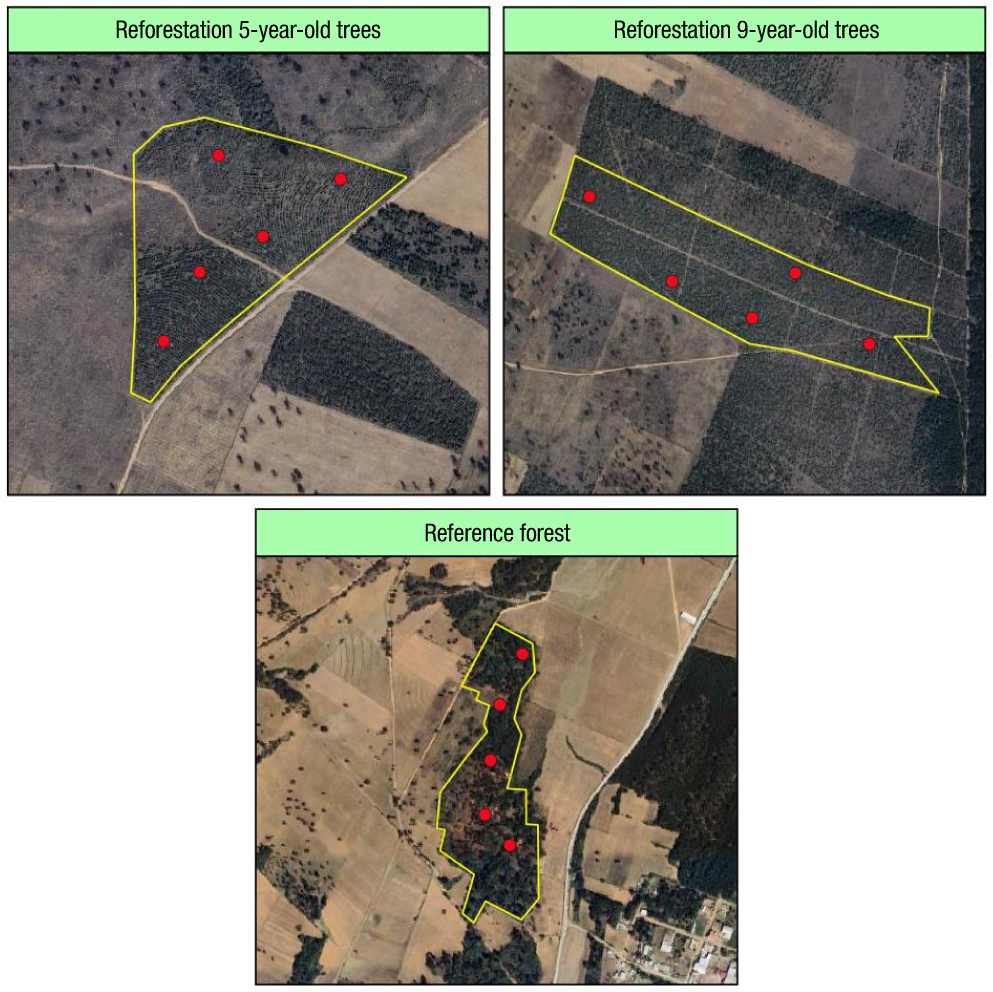
Using random sampling and a point grid spaced at 100 m intervals, five circular plots of 400 m2 were established in each zone (Figure 3). Within these plots, tree measurement parameters were measured, including diameter at breast height (DBH), using a diameter tape (Forestry Suppliers Inc.), and total tree height (H), using an 8-meter telescopic stadia rod (Hastings). For taller trees, a digital clinometer (Haglöf) was used.
In all three study areas, height and diameter were measured for all individuals with a DBH ≥ 2.5 cm (Alanís-Rodríguez et al., 2020). Diameter and height distributions for each zone were represented using frequency histograms. Basal area was calculated using the formula: AB (m2) = π (DBH2) / 4.
Tree volume was estimated using the models applied by UMAFOR-2103-Teziutlán, as indicated in Table 1 (Ingeniería Agroforestal y Ambiental del Bosque Mesófilo [INAFAM], 2015).
Table 1.
| Species | Models |
|---|---|
| Vol = Exp [-9.63495649 + 1.86670523 Ln (DBH) + 0.99551381 Ln (H)] | |
| Vol = Exp [-9.73084158 + 1.86001307 Ln (DBH) + 0.98860113 Ln (H)] | |
| Vol = Exp [-9.69246238 + 1.92883177 Ln (DBH) + 0.90538711 Ln (H)] |
Tree density was estimated by averaging the number of individuals found in the five 400 m2 sampling plots per study area and extrapolating the results to individuals per hectare. The Importance Value Index (IVI), which ranks the dominance or ecological importance of one species relative to others (Graciano-Ávila et al., 2020; Mendoza-Aguirre et al., 2021), was calculated only for the tree community in the reference forest (RF), as P. montezumae was the sole species present in the reforested areas. The IVI was calculated using the equations developed by Curtis and Mclntosh (1951):
where,
Relative density was estimated as follows:
Relative frequency was estimated as follows
Statistical analysis
The data met the assumptions of normality (Shapiro-Wilk test) and homogeneity of variances (Bartlett’s test), so data transformation was not necessary. To determine whether statistically significant differences existed in tree measurement parameters among areas, an ANOVA was performed (α = 0.05), followed by a Tukey’s post hoc test for multiple comparisons (P = 0.05) using the R software within the RStudio platform (The R Core Team, 2022).
Results and Discussion
Diameter and height classes
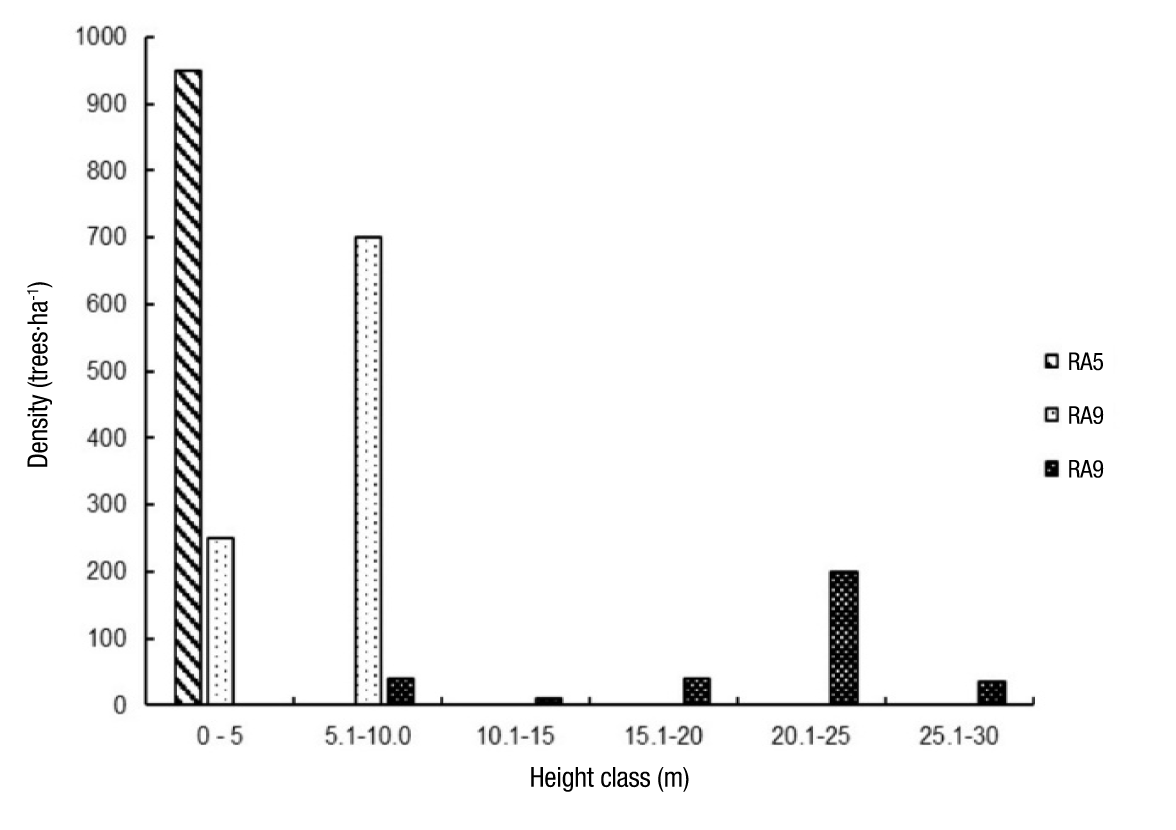
Diameter and height classes showed significant differences (p ≤ 0.05) among the study areas, with RA5 exhibiting the lowest values. In the two P. montezumae reforestation sites, the average tree diameter (Figure 4) ranged from 5.8 cm (RA5) to 11.2 cm (RA9), and the average height (Figure 5) varied from 2.5 m (RA5) to 4.4 m (RA9). The reference forest exhibited the greatest diameter (39.8 cm) and height (18.1 m), indicating that the stand corresponds to a mature forest (Figures 6 and 7).
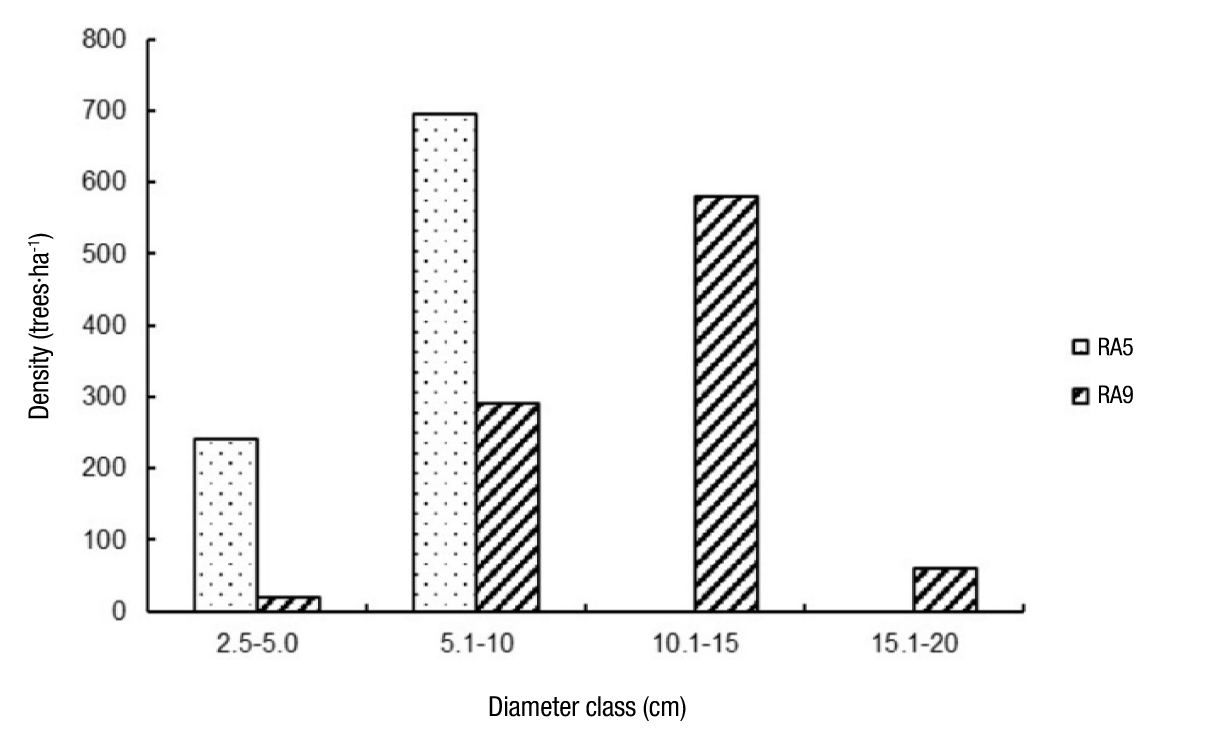
RA5 and RA9 are in an early developmental stage (5-20 cm), corresponding to the monte bravo and vardascal stages. These stands must progress through additional successional stages before achieving the structural characteristics of mature forests (fustal) (Aguilar-Luna, 2018). These changes are largely influenced by microclimatic conditions. As forest structure becomes more complex, it affects temperature and humidity and increases the availability of resources (water and nutrients), which in turn promotes understory vegetation growth (Gadow et al., 2012).
In the reference forest, nine diameter classes were recorded, ranging from 15 to 65 cm DBH, with P. teocote showing the highest number of individuals in the 40-65 cm diameter range (Figure 6).
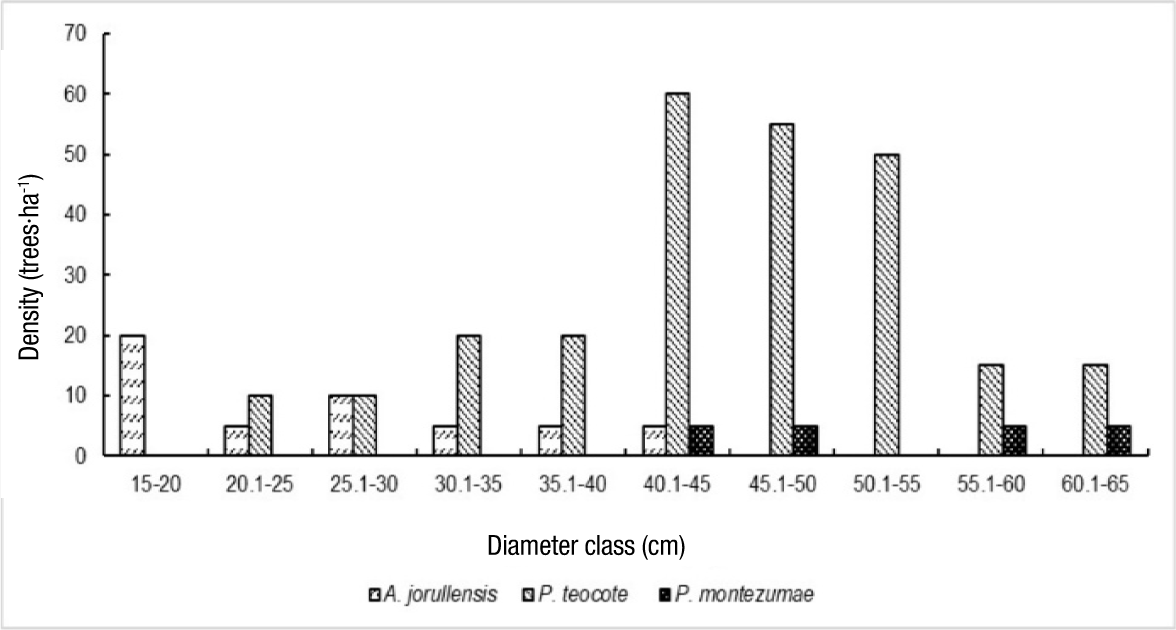
In the reference forest, the highest number of trees was observed in the diameter classes >40 cm, indicating the presence of two developmental stages: vardascal and fustal. Typically, in a mature forest that is undisturbed and maintains continuous natural regeneration, tree density tends to be concentrated in the lower diameter classes and gradually decreases (Bhutia et al., 2019), resulting in an inverted ‘J’-shaped distribution (Aguirre-Mendoza et al., 2021). This pattern was not observed in the reference forest (Figure 6). A possible explanation for the observed pattern may be related to the presence of nearby communities that engage in various activities within the forest, particularly livestock grazing. Grazing contributes to soil compaction and mortality of natural regeneration due to browsing, both of which negatively affect forest regeneration (Gadow et al., 2012).
In terms of height, in RA5 the highest number of individuals was observed in the 0-5 m category, whereas in RA9 most individuals were found in the 5.1-10 m category (Figure 5). The average height in RA5 was 2.5 m, while in RA9 it was 4.4 m. In the reference forest, which contains a greater diversity of tree species, P. montezumae had an average height of 23.4 m, P. teocote averaged 22.2 m, and A. jorullensis reached an average height of 8.9 m (Figure 7).
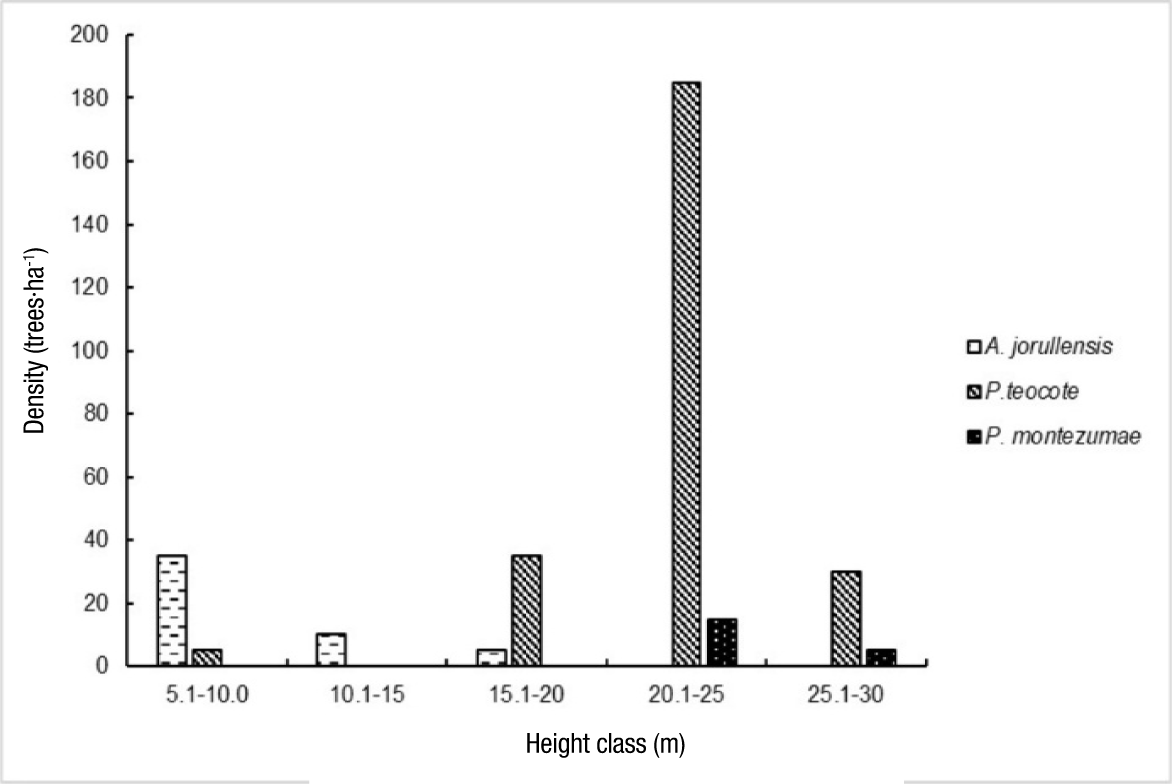
Both species identity and the environmental and physical conditions of the planting site influence the number of surviving individuals and their development (Torres-Rojo, 2021). In plantations of P. montezumae aged between 7 and 32 years in Nuevo San Juan Parangaricutiro, Michoacán, average heights of 9.2 m have been reported (Hernández Ramos et al., 2024), which are higher than those observed in RA5. That site presents only one height class (0-5 m), while RA9 shows two classes-fewer than those found in the reference forest, which displays five height classes (Figure 6). This variation in height is a key attribute of vertical structure and is useful for assessing structural tree diversity (Martínez-Sánchez, 2016). Vertical structural diversity is highly important for biodiversity, its processes, and functions, as it is closely linked to microhabitat conditions such as humidity, light availability, and temperature (Martínez-Sánchez, 2016).
The lower complexity in the vertical structure of reforested areas during the early years of establishment may not have a significant immediate effect on the previously mentioned ecological processes. Therefore, it is necessary to allow these species to reach reproductive maturity in order to initiate natural regeneration processes, which over time can lead to increased vertical and horizontal structural diversity. This, in turn, will have a greater impact on biodiversity, as well as on ecosystem processes and functions in reforested areas. This does not mean that reforestation is unimportant; rather, it suggests that some of its outcomes will only become evident in the medium to long term. Although reforested areas may initially lack complex vertical and horizontal structure, they still fulfill other essential ecological functions, such as soil retention, reduction of surface runoff and erosion, provision of habitat for plant and animal species, rainwater interception (through stems, foliage, and branches), and microclimate modification on a different scale than that associated with higher structural diversity.
Structural characteristics
Basal area has been used as an indicator for assessing the degree of forest recovery (Graciano-Ávila et al., 2020), and it is an essential attribute for understanding forest ecosystems (Bhutia et al., 2019). In the present study, statistical analysis of basal area, volume, and density revealed significant differences (p ≤ 0.05) among the three sites (Table 2). It was observed that as the age of the reforestations increases, both basal area and volume also increase. The basal area of a forest reflects the diameter growth behavior of trees and the effects of stand age. According to Graciano-Ávila et al. (2020), forests tend to increase their basal area asymptotically over time, resembling the pattern found in undisturbed forests. Moreover, the increase in basal area is important not only for timber production but also as an indicator of greater plant and animal species diversity. It is also a valuable metric for understanding aboveground biomass production and, indirectly, carbon secuestration and storage (Luna-Florín et al., 2021)-an ecosystem service inherent to forests and reforested areas.
Table 2.
| Variables | RA5 | RA9 | RF |
|---|---|---|---|
| Basal area (m2∙ha-1) | 2.64 c | 10.11 b | 49.01 a |
| Volume (m3∙ha-1) | 4.01 c | 25.11 b | 238.14 a |
| Density (trees∙ha-1) | 935 a | 950 a | 325 b |
Means followed by different letters are significantly different between zones according to Tukey’s test (p ≤ 0.05).
Stem volume in the reforested areas, like basal area, tends to increase with stand age. In the case of the reference forest, tree volume was 238.14 m3∙ha-1, a value higher than those recorded in RA5 and RA9. Arteaga-Martínez (2003) reported a volume of 39.8 m³∙ha-1 in P. montezumae plantations aged 15 years, exceeding the value obtained in RA9 by 37 %; however, RA9 shows a higher average annual increment (2.79 vs. 2.65 m3∙ha-1).
Reforestations RA5 (935 trees∙ha-1) and RA9 (950 trees∙ha-1) exhibited significantly higher tree density than the reference forest (325 trees∙ha-1) (Table 3). In reforested areas, initial survival is influenced by plant handling, nursery seedling quality, seedling transport, field management practices, and genetic quality and persistence (Torres-Rojo, 2021). The higher density observed in the reforestation areas compared to the reference forest is largely a result of the initial planting density. Reforestation areas efforts typically involve planting densities of around 1 100 seedlings∙ha-1 (Prieto-Ruiz et al., 2016; Vanegas-López, 2016). In these areas, both biotic and abiotic conditions-such as soil properties and microclimate-are fundamental for seedling survival and species development (Torres-Rojo, 2021). In the reference forest, tree density was variable, similar to findings in other studies. For example, Hernández-Ramos et al. (2024) also reported wide variability, ranging from 175 to 1 000 individuals∙ha-1. Tree density in the reference forest is determined by several factors, including the availability of germplasm, dispersal syndrome, favorable conditions for seed germination and seedling emergence, predation, pests and diseases, competition, and stand age. Additionally, anthropogenic disturbances-due to the forest’s proximity to rural human settlements-represent a negative factor impacting the density of remnant forests.
Table 3.
| Species | N (trees∙ha-1) | Relative density | Relative dominance | Relative frequency | IVI (%) |
|---|---|---|---|---|---|
| 50 | 15.4 | 6.0 | 41.7 | 21.00 | |
| 20 | 6.2 | 8.8 | 16.7 | 10.53 | |
| 255 | 78.5 | 85.3 | 41.7 | 68.47 | |
| 325 | 100 | 100 | 100 | 100 |
In the reference forest, P. teocote had the highest IVI (68.47 %), followed by A. jorullensis with 21 %, and P. montezumae with 10.53 % (Table 3). The IVI results for the reference forest agree with previous reports on temperate forests in Mexico, where the genus Pinus is typically the most representative, often displaying dominant tree-measurement parameters and, consequently, a high IVI (Domínguez-Gómez et al., 2018; López-Hernández et al., 2017; Silva-García et al., 2022). IVI can serve as an ecological tool for selecting species to reforest degraded or deforested areas. In the reference forest, P. teocote had the highest IVI, and it would therefore be expected that reforestation efforts within the ejido areas would have prioritized this species. However, the species most commonly used for reforestation was P. montezumae. Local people prefer this species because of its higher wood quality and commercial value, as well as its resistance to frost, pests, diseases, and wildfires. Another decisive factor is the ease of obtaining seedlings through government programs. Given these considerations, further structural studies in surrounding forests are recommended to determine whether similar IVI patterns occur as those observed in this study.
Conclusions
Structural attributes are essential for evaluating reforestation efforts, particularly when these are used as a strategy for forest restoration. These attributes change over time as forest structure becomes more complex; however, in the short term-as in this study (five and nine years)-it is not yet possible to conclude that reforested areas resemble the reference forest. The results are not definitive, underscoring the need for continued monitoring and evaluation of these reforestations over the medium and long term to gain a more comprehensive understanding of changes in structural parameters. Furthermore, beyond structural attributes, it is important to include studies on biodiversity, ecosystem functions, and ecological processes, which may require much longer timeframes to fully assess the role of reforestation in restoring all ecosystem components.