

Introduction
Cacao (Theobroma cacao L.) is a perennial crop of great importance in Mexico and across tropical regions worldwide. In Mexico, 52 449 ha are cultivated in the southeastern region, specifically in the states of Oaxaca, Chiapas, and Tabasco, the latter accounting for 61 % of national production (Servicio de Información Agroalimentaria y Pesquera [SIAP], 2023).
In Tabasco, several insect pests have been reported affecting T. cacao. Among the most prominent are the hibiscus mealybug (Maconellicoccus hirsutus Green) (Torres de la Cruz et al., 2019), the spittlebug (Clastoptera laenata Fowler), the whitefly (Lecanoideus floccissimus Martin), the cacao moth (Hemeroblema mexicana Guenée), the red-banded thrips (Selenothrips rubrocinctus Giard), the black aphid (Toxoptera aurantii Boyer de Fonscolombe), and the borer Xyleborus vulvulus Fabricius (Sánchez-Soto & Cortez-Madrigal, 2000). These pests reduce both the quality and yield of cacao production.
Recently, the black stink bug (Antiteuchus tripterus Fabricius, 1787) (Hemiptera: Pentatomidae) has been reported in cacao plantations in Tabasco. This insect is a significant pest of cacao in several Caribbean and South American countries, including Trinidad and Tobago, Brazil, Ecuador, and Peru (Castillo-Carrillo et al., 2020). Damage is caused by both nymphs and adults, which feed by sucking sap from the peduncles and the base of the fruits. During feeding, the black stink bug injects toxins that lead to wilting and death of fertilized flowers, known locally as chilillos. In developing fruits, the bug causes shallow lesions that can extend from the peduncle to the apex, potentially creating entry points for phytopathogenic fungi. Additionally, Castillo-Carrillo et al. (2020) reported that this insect acts as a mechanical vector of cacao frosty pod rot (Moniliophthora roreri [Cif. & Par.] Evans et al., 2003). Consequently, the development of effective and sustainable management strategies for this pest is urgently needed.
Chemical control of A. tripterus can significantly reduce insect populations; however, the use of synthetic insecticides may contribute to resistance development, leave harmful residues on the fruit, and negatively impact key cacao pollinators (Pu & Chung, 2024). In the search for environmentally friendly alternatives, biological control offers a sustainable option. In this regard, entomopathogenic fungi such as Metarhizium anisopliae (Metschn.) Sorokin, Beauveria bassiana (Bals.-Criv.) Vuill., and Paecilomyces lilacinus (Thom) Samson have demonstrated effectiveness against A. tripterus in Colombia (Yepes-Rodríguez, 2019). Despite the presence of A. tripterus in Mexican cacao plantations, there are no reports of native entomopathogenic fungi with proven biological efficacy for controlling this insect. Therefore, the objective of this study was to characterize and select native isolates of Metarhizium spp. for the biological control of the black stink bug (A. tripterus) in cacao plantations in Tabasco, Mexico. This research contributes to the understanding of entomopathogenic fungal diversity and proposes a biological control alternative for managing A. tripterus in cacao crops in Tabasco.
Materials and Methods
Collection site
Adults of A. tripterus infected with entomopathogenic fungi were obtained through targeted sampling in a cacao plantation located in the community of José María Morelos y Pavón (Las Delicias), Teapa, Tabasco. The collection site is located at coordinates 17° 38' 5.1" N, 92° 55' 48.2" W, an elevation of 10 meters. Mycosed cadavers were transferred into sterile vials, placed in thermal containers, and transported to the Entomopathogen Laboratory at the Academic Division of Biological Sciences, Universidad Juárez Autónoma de Tabasco.
Isolation of fungal strains
A. tripterus cadavers were sterilized in a 0.5 % sodium hypochlorite solution for 5 minutes, following the protocol described by Gerónimo-Torres et al. (2016). They were then rinsed with sterile distilled water (SDW) and individually placed in humid chambers at 25 °C for 8 days for sporulation. Sporulating cadavers were used to inoculate Sabouraud Dextrose Agar supplemented with 0.1 % yeast extract (SDA + YE). Monospore isolates were obtained from polysporic cultures using the method described by SENASICA (Servicio Nacional de Sanidad, Inocuidad y Calidad Agroalimentaria, 2016). The isolates were stored under refrigeration until specific characterization assays.
Morphological identification
The fungal isolates were identified to the species level based on their reproductive structures, following the criteria described by Barnett and Hunter (1998) and Bischoff et al. (2009). For morphological characterization, the isolates were grown on Petri dishes containing SDA + YE medium for 14 days. Colony characteristics such as size, morphology, and conidiation were recorded for each isolate. Additionally, a spore suspension was inoculated onto 0.5 cm SDA discs placed under sterile coverslips to observe the microscopic structures of each isolate. The inoculated discs were incubated in a humid chamber at 25 °C for 3 to 5 days. Microscopic characteristics of the conidiophores and conidia were observed using an Axio Scope A1 brightfield optical microscope (Carl Zeiss, Microscopy GmbH®, Göttingen, Germany), and images were captured with an AxioCam ERc5s digital camera (Carl Zeiss®). Morphometric data of the reproductive structures were obtained using the measurement tools of the Zen/2011 software (Carl Zeiss Microscopy GmbH®). The isolates were deposited in the entomopathogenic fungi collection of the Entomopathogen Laboratory at the Academic Division of Biological Sciences, Universidad Juárez Autónoma de Tabasco, Villahermosa, Tabasco, Mexico.
Molecular identification
Genomic DNA was extracted from 7-day-old pure cultures using the CTAB (cetyltrimethylammonium bromide) method, and DNA concentration was estimated with a NanoDrop 2000 spectrophotometer (Thermo Scientific®). For phylogenetic analysis, partial gene sequences from two regions were amplified by PCR: the nuclear rDNA ITS1-5.8S-ITS2 region and the β-tubulin gene. The ITS region was amplified using primers ITS5 (5′-gca agt aaa agt cgt aac aag g-3′) and ITS4 (5′-tcc tcc gct tat tga tat gc-3′). Partial amplification of the β-tubulin gene was performed using primers Bt2a (5′-ggt aac caa atc ggt gct gct ttc-3′) and Bt2b (5′-acc ctc agt gta gtg acc ctt ggc-3′). PCR reactions for both genes were carried out under the following conditions: initial denaturation at 94 °C for 2 min; 40 cycles of 94 °C for 30 s, 55 °C for 45 s, and 72 °C for 90 s; followed by a final extension at 72 °C for 4 min. Each 25 µL PCR reaction contained 1X buffer, 1.5 mM MgCl₂, 0.2 mM dNTPs, 0.4 µM of each primer (Integrated DNA Technologies, Inc.), 1 U of Taq DNA polymerase (Promega), and 20 ng of genomic DNA. DNA quantification was performed using a NanoDrop 2000 (Thermo Scientific®). Amplicons were submitted for sequencing to Psomagen Inc. (USA). The resulting sequences were compared with those available in GenBank using BLASTn (Basic Local Alignment Search Tool for nucleotides) at the National Center for Biotechnology Information (NCBI, https://www.ncbi.nlm.nih.gov/).
Phylogenetic analysis
A total of 24 taxa previously downloaded from NCBI were used, including the sequences obtained from the isolates. DNA sequences were aligned using MUSCLE, implemented in MEGA-X (Kumar et al., 2018), and concatenated with SeaView 4.7 (Gouy et al., 2010). The best-fit nucleotide substitution model was determined using jModelTest v2 (Darriba et al., 2012), based on the Akaike Information Criterion (AIC). Phylogenetic analysis was conducted using IQ-TREE v2 (Minh et al., 2020), which implements a maximum likelihood algorithm, through the CIPRES Science Gateway v3.3 portal (https://www.phylo.org/portal2/login!input.action). The resulting phylogenetic tree was visualized and edited using iTOL (Letunic et al., 2021).
Physiological characterization
Mycelial growth
Five-day-old cultures of each isolate were used to transfer a 5 × 5 mm section from the edge of the colony onto a 90 mm Petri dish containing SDA + YE medium, using a sterile cork borer. The inoculated plates were incubated at 25, 30, and 35 ± 1 °C to evaluate the thermal tolerance of the fungus. Each treatment included five replicates per isolate and temperature. Mycelial growth (MG) was recorded every 2 days until one of the isolates fully covered the medium. The average radial growth (RG) on the final day was used for statistical analysis. The effect of temperature on RG was assessed by calculating the percentage of growth increase (INC) or inhibition (INH) using the following formulas: % (INH/INC) = [(RG at 30 °C x 100/RG at 25 °C) - 100], and % (INH/INC) = [(RG at 35 °C x 100/RG at 30 °C) - 100], according to Torres-de la Cruz et al. (2013).
Germination rate
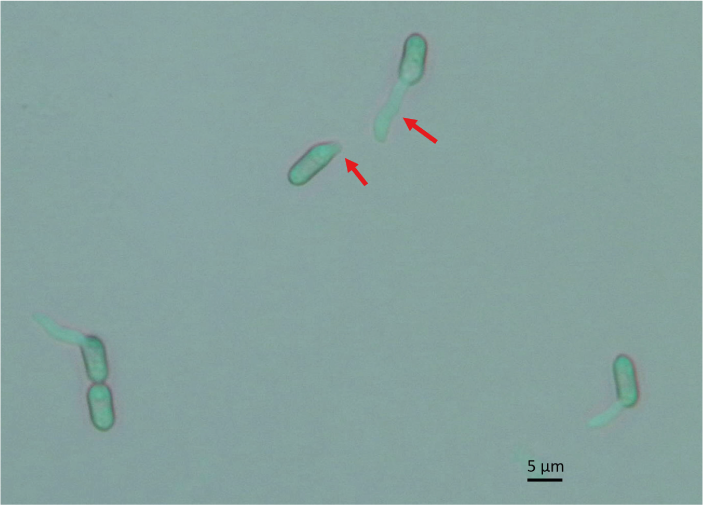
Eighteen-day-old cultures of each isolate were used to prepare a conidial suspension at a concentration of 5 × 10⁶ conidia∙mL⁻¹. From this suspension, 30 µL were deposited onto Petri dishes containing SDA + YE medium. Four replicates were established per treatment. The plates were incubated at three temperatures: 25, 30 and 35 °C ± 1 °C. Germination was monitored by examining 100 conidia per replicate at hourly intervals under a light microscope, continuing until one of the isolates reached 90 % germination. Conidia were considered germinated when the germ tube length was at least half the length of the conidium (Figure 1).
Conidial production on SDA medium
From each fungal isolate, 5 × 5 mm sections were taken from the actively growing edge of 8-day-old colonies using a sterile cork borer and transferred to Petri dishes containing SDA + YE medium. The plates were incubated at 25, 30, and 35 ± 1 °C for 16 days in the dark. Conidia were harvested by flooding the culture with sterile distilled water (SDW) containing 0.1 % Tween 80 and gently scraping the spores with a stainless steel micro-spatula. The resulting conidial suspension was homogenized for 1 min using a magnetic stirrer. To separate conidia from mycelial fragments, the suspension was filtered through sterile medical gauze (Protec®, 20 × 12 pads). Conidial production (CP) per isolate (five replicates) was estimated with a Neubauer chamber. The number of conidia∙mL-1 was calculated by the formula C = (Cc) (4 x 10⁶) (Fd/80); where, Cc = the average number of conidia counted in five quadrants of the Neubauer chamber, and Fd = dilution factor.
The effect of temperature on CP in SDA medium was evaluated by calculating the percentage of inhibition or increase in CP when shifting from 25 to 30 °C and from 25 to 35 °C, using the following formulas: % INH/INC = [(CP at 30 °C x 100/ CP at 25 °C) -100] and % INH/INC = [(CP at 35 °C x 100/ CP at 25 °C)-100] (Torres-de la Cruz et al., 2013).
Conidial production on rice
Thirty grams of rice were placed in a polypaper bag and moistened with 7 mL of distilled water. The bags were then sterilized at 121 °C for 20 minutes. After cooling, each bag was inoculated with 5 mL of a conidial suspension at a concentration of 1 × 10⁷ conidia∙mL-1 and incubated for 16 days at 25 ± 1 °C under a 12:12 h light:dark photoperiod. Five replicates were established per isolate. At the end of the incubation period, the 30 g of rice were transferred to 150 mL of sterile distilled water containing 0.1 % Tween 80. The mixture was agitated for 10 minutes and filtered through sterile medical gauze. The total number of conidia per isolate was estimated using a Neubauer hemocytometer. Conidial production per gram of rice was calculated using the same formula applied for conidial production on SDA medium (Torres-de la Cruz et al., 2013).
Pathogenic characterization
Adults of A. tripterus were collected using small sweep nets in the same cacao plantation where the mycosed insects had previously been found. Captured insects were placed in plastic containers covered with mesh lids. As a food source, an immature T. cacao fruit approximately 8 cm in length was placed inside each container. The insects were then transported to the Entomopathogen Laboratory at the Academic Division of Biological Sciences, Universidad Juárez Autónoma de Tabasco.
In the laboratory, live insects were immersed for 1 minute in a conidial suspension of 1 × 10⁷ conidia·mL-1 + 0.1 % Tween 80. Five Metarhizium isolates and one control treatment were evaluated. For the control group, insects were submerged in sterile distilled water (SDW) containing 0.1 % Tween 80. Treated adults were placed in plastic containers with mesh lids. TenA. tripterusadults constituted one experimental unit, with five replicates per fungal isolate. A juvenile cacao pod measuring 8 cm was placed inside each container as a food source. The treated specimens were maintained at 25 ± 1 °C, and humidity was regulated using ADE-moistened cotton wads. Mortality was recorded daily, and dead insects were transferred to a humid chamber to promote sporulation. The effectiveness (EF) of each fungal isolate was determined using mortality data and the formula: % EF = [(Mtest - Mtrat) / Mtest] x 100; where Mtest and Mtrat represent mortality in the control and Metarhizium treatment, respectively. Mortality in the control treatment was factored into the formula.
Statistical analysis
Data on mycelial growth, conidial production on SDA medium and rice, and pathogenicity (effectiveness) were analyzed using a completely randomized design with five treatments (isolates). Prior to analysis, mortality data were transformed using the arcsine square root of the proportion. Mycelial growth and conidial production data (on SDA and rice) were log-transformed using the formula log (x + 1). Subsequently, treatments were compared through ANOVA (P ≤ 0.05), followed by Tukey’s multiple comparison test using SAS software, version 9.0 (SAS Institute Inc.). The time required to reach 50 and 90 % conidial germination (TG₅₀ and TG₉₀) was estimated using Probit analysis (SAS Institute Inc.).
Results and Discussion
Morphological and molecular characterization
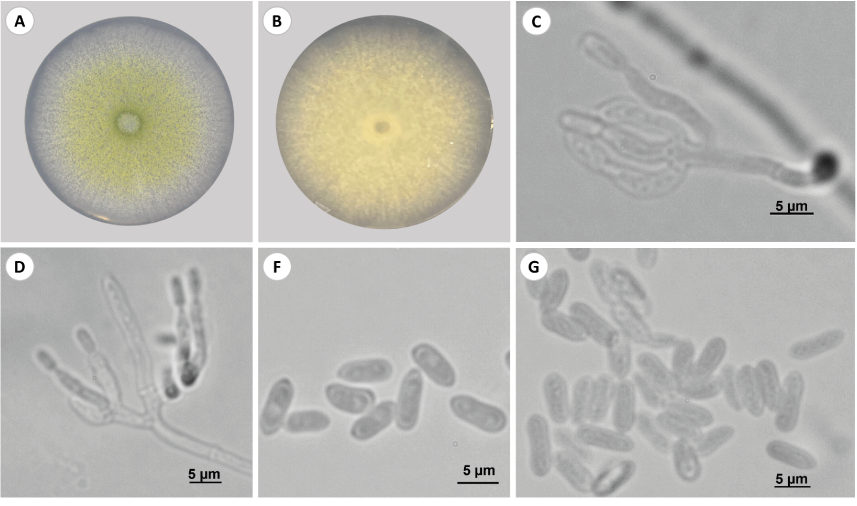
A total of five fungal isolates were obtained from A. tripterus adults naturally infected under field conditions: TCCH2, TCCH5, TCCH7, TCCH8, and TCCH9. Figure 2 shows some morphological features of the fungus. All isolates formed circular colonies with a flat surface, variable texture, and initially white coloration that turned olive green to dark green as the conidia matured (Figure 2 A-B). The conidiophores were hyaline and branched, bearing phialides singly, in pairs, or in whorls (Figure 2 C-D). Conidia were produced in basipetal chains, cylindrical in shape, hyaline or slightly pigmented, and aggregated in olive-green masses (Figure 2 E-F). These characteristics are consistent with descriptions for the genus Metarhizium as reported by Barnett and Hunter (1998). The conidia measured 5-8.15 × 2-3.08 µm (Table 2), which falls within the range described for M. anisopliae by Bischoff et al. (2009). However, these authors noted that five Metarhizium species-M. anisopliae, M. brunneum Petch, M. lepidiotae (Driver & Milner) J. F. Bisch., S. A. Rehner & Humber, M. pingshaense Q. T. Chen & H. L. Guo, and M. robertsii J. F. Bisch., S. A. Rehner & Humber-overlap in conidial size and morphology. Therefore, species-level identification cannot be reliably determined based on conidial morphology alone.
Isolates TCCH5, TCCH7, and TCCH8 were identified through sequencing of ITS and β-tubulin. The sequences for these isolates were deposited in GenBank: TCCH5 (accession number: PP948902), TCCH7 (accession numbers: PP938692 and PP948903), and TCCH8 (accession number: PP938693). The phylogenetic tree constructed with sequences from the three Metarhizium isolates and additional Metarhizium species sequences retrieved from GenBank is shown in Figure 3. The bootstrap analysis revealed well-supported main branches that clearly separated the sequences of the species used. Based on significant bootstrap values, the sequences from the three native Metarhizium isolates in this study grouped into a single clade with the type and reference strains of M. brunneum, with a bootstrap support of 88 %. The species M. brunneum has also been reported in other countries and from insect hosts across various orders, including Coleoptera, Diptera, Isoptera, Hymenoptera, Lepidoptera, Orthoptera, and Hemiptera (Bischoff et al., 2009). Within Hemiptera, M. brunneum has been reported on the stink bug Euschistus heros (Pentatomidae) (Resquín-Romero et al., 2020), the olive fruit fly Bactrocera oleae (Diptera: Tephritidae) (Yousef et al., 2013), and the wireworm Agriotes spp. (Razinger et al., 2018). This is the first report of M. brunneum infecting A. tripterus (Pentatomidae).
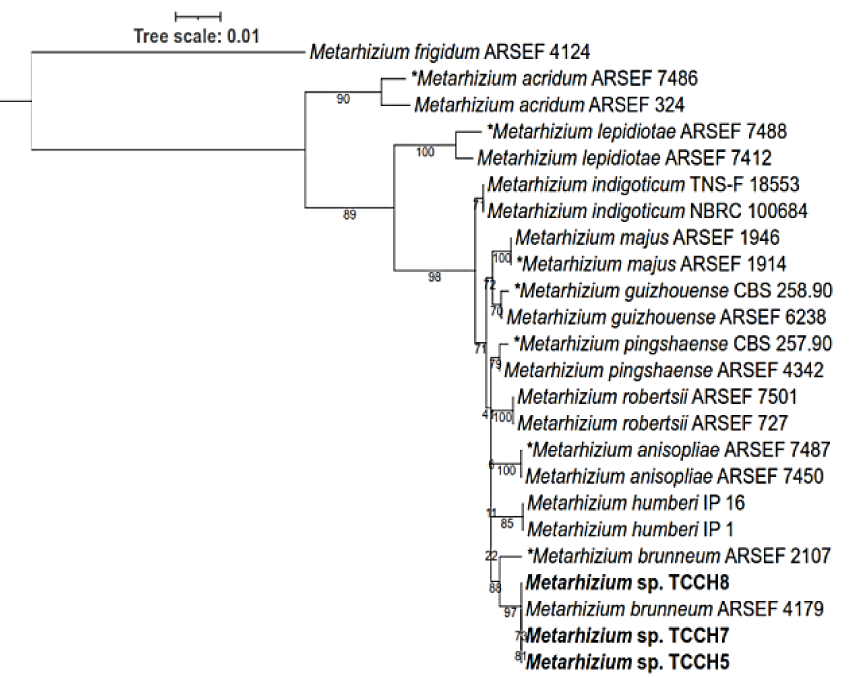
Table 1.
| Strains | Mycelial growth (mm) | Inhibition (-) or increase (+) (%) | |||
|---|---|---|---|---|---|
| 25 °C | 30 °C | 35 °C | 25-30 °C | 25-35 °C | |
| TCCH2 | 16.46 ± 0.24 ab | 5.81 ± 0.77 a | 0 | -64.70 | -100 |
| TCCH5 | 16.32 ± 0.30 b | 5.42 ± 0.44 a | 0 | -66.79 | -100 |
| TCCH7 | 16.75 ± 0.49 ab | 5.17 ± 0.19 a | 0 | -69.13 | -100 |
| TCCH8 | 17.27 ± 0.69 a | 5.33 ± 0.17 a | 0 | -69.14 | -100 |
| TCCH9 | 17.21 ± 0.35 a | 5.80 ± 0.34 a | 0 | -66.30 | -100 |
Means (± standard deviation) followed by different letters in a column are statistically different according to Tukey’s test (P < 0.05)
Physiological characterization
Mycelial growth
Table 1 shows the results of mycelial growth for the fungal isolates at the three tested temperatures. At 25 °C, significant differences were observed among isolates (P < 0.0085); the highest mycelial growth was recorded for isolates TCCH8 (17.27 mm) and TCCH9 (17.21 mm), while TCCH5 showed the lowest growth (16.32 mm), although it was not significantly different from TCCH7 and TCCH2. At 30 °C, growth ranged from 5.17 to 5.81 mm, and no significant differences were observed among isolates (P < 0.1044). However, all isolates showed a marked reduction in growth, with decreases ranging from 64.7 % to 69.1 % compared to their growth at 25 °C. These findings differ from those reported by Torres-de la Cruz et al. (2013), who found growth inhibition ranging from 0 to 27 % in native isolates of M. anisopliae under similar conditions. At 35 °C, mycelial growth was completely inhibited (100 %) for all isolates. In contrast, Torres-de la Cruz et al. (2013) reported inhibition levels between 74.1 % and 86.3 % for M. anisopliae at the same temperature. Based on these results, the optimal temperature range for mycelial growth of the native M. brunneum isolates was between 25 and 30 °C, consistent with previous reports for M. anisopliae (Torres-de la Cruz et al., 2013). Similarly, Ortiz-Catón et al. (2011) noted that the optimal development of entomopathogenic fungi typically occurs between 20 and 28 °C. The thermal performance of M. brunneum in this study may be attributed to the tropical origin of the isolates. Moreover, Gebremariam et al. (2021) emphasized the importance of mycelial growth as a key criterion in selecting promising isolates for biological control applications.
Germination rate
According to Table 2, variability was observed in the germination rate of M. brunneum, both among isolates and temperatures. At 25 °C, the isolates with the highest and lowest TG50 were TCCH2 (8.8 h) and TCCH9 (7.8 h), respectively. These results are similar to those reported by -de la Cruz et al. (2013), who documented TG50 values ranging from 7.4 to 8.2 h for native isolates of M. anisopliae incubated at 25 °C. However, the TG50 values reported for M. brunneum in the present study are lower than those reported for native isolates of Beauveria bassiana (12.6 to 15.9 h) by Gerónimo-Torres et al. (2016). At 30 °C, the highest TG50 was observed in strain TCCH5, with 9.5 h, while the lowest TG50 was recorded for strain TCCH2, with 7.8 h. Notably, TCCH2 showed a reduced germination time compared to TG50 at 25 °C. When TG50 was assessed at 35 °C, all strains showed an increase in germination time, similar to that reported by Torres-de la Cruz et al. (2013) for M. anisopliae. At this temperature, the strain with the highest TG50 was TCCH2, with 21.9 h, while strains TCCH5, TCCH7, and TCCH8 had the lowest TG50 values.
Table 2.
| Strains | 25 °C | 30 °C | 35 °C | |||||
|---|---|---|---|---|---|---|---|---|
| Average (h) | RV | Average (h) | RV | Average (h) | RV | |||
| TCCH2 | 8.8 | 8.6-9.1 | 7.8 | 7.8-8.0 | 21.9 | 18.6-38.5 | ||
| TCCH5 | 8.3 | 8.1-8.6 | 9.5 | 9.3-9.7 | 12.7 | 12.7-12.9 | ||
| TCCH7 | 8.2 | 8.1-8.3 | 8.6 | 8.5-8.9 | 13.8 | 13.7-13.9 | ||
| TCCH8 | 8.5 | 8.2-8.8 | 8.5 | 8.3-8.7 | 14.1 | 13.9-14.4 | ||
| TCCH9 | 7.8 | 7.5-8.1 | 8.0 | 7.9-8.1 | 15.0 | 14.8-15.3 | ||
Regarding TG90, at 25 °C, the strain with the longest germination time was TCCH8 (10.9 h), while the strain with the shortest time was TCCH9 (9.6 h) (Table 3 ). At 30 °C, the strains with the highest and lowest TG90 were TCCH5 and TCCH2, with 12.3 h and 9.5 h, respectively. Similarly, at 35 °C, these two strains maintained the highest and lowest TG90 values, with 27.7 h and 14.6 h, respectively. At this temperature, all strains showed an increased germination time compared to TG90 at 30 °C; however, strains TCCH5, TCCH7, and TCCH8 showed the lowest TG90 values. Although all M. brunneum isolates germinated at 25 and 35 °C, the optimal temperature range for conidial germination in these strains is between 25 and 30 °C (Tables 2 and 3). According to Faria et al. (2015), germination speed is also a relevant factor in the selection of efficient strains for use as biological control agents.
Table 3.
| Strains | 25 °C | 30 °C | 35 °C | |||||
|---|---|---|---|---|---|---|---|---|
| Average (h) | RV | Average (h) | RV | Average (h) | RV | |||
| TCCH2 | 10.7 | 10.3-11.4 | 9.5 | 9.3-9.7 | 27.7 | 21.6-64.6 | ||
| TCCH5 | 10.5 | 10.0-11.3 | 12.3 | 11.8-12.9 | 14.6 | 14.4-14.8 | ||
| TCCH7 | 9.7 | 9.6-9.9 | 10.9 | 10.5-11.6 | 15.6 | 15.4-15.9 | ||
| TCCH8 | 10.9 | 10.3-12.1 | 10.9 | 10.4-11.5 | 16.1 | 15.7-16.7 | ||
| TCCH9 | 9.6 | 9.1-10.3 | 10.0 | 9.8-10.3 | 17.4 | 16.9-18.1 | ||
Conidial production on SDA + YE medium
According to Table 4, at 25 °C, no significant differences were observed (P < 0.3340) in conidial production on SDA + YE medium. However, the isolates with the highest production were TCCH2 and TCCH9, with 9.7 × 10⁷ and 9.0 × 10⁷ conidia∙mL⁻¹, respectively. These levels of conidial production are similar to those reported by Valle-Ramírez et al. (2022) for Metarhizium spp. isolates. At 30 °C, significant differences were observed among isolates (P < 0.0008); the strains with the highest conidial production were TCCH8 and TCCH9, with 1.5 × 10⁷ and 7.5 × 10⁶ conidia∙mL⁻¹, respectively, while the lowest production was recorded for TCCH7, with 3.7 × 10⁶ conidia∙mL⁻¹ (Table 4). At this temperature, conidial production on SDA + YE medium decreased by 76.2 % to 94.7% compared to the levels observed at 25 °C, with strain TCCH8 being the least affected by temperature. Isolates incubated at 35 °C showed neither mycelial growth nor conidial production. Gerónimo-Torres et al. (2016) reported a reduction in conidial production in native isolates of B. bassiana when incubated from 25 to 30 °C, and also observed no mycelial growth or conidial production at 35 °C. Therefore, the effective temperature range for sporulation in native M. brunneum strains was 25 to 30 °C; however, the optimal temperature was 25 °C.
Table 4.
| Strains | Rice (25 °C) (conidia∙g-1) |
SDA +YE (25 °C) (conidia∙mL-1) |
SDA + YE 30 °C (conidia∙mL-1) |
Inhibition (-)/Increase (+) (%) | |
|---|---|---|---|---|---|
| 25-30 °C | 25-35 °C | ||||
| TCCH2 | 1.98 x 10⁸ ± 1.6 x 10³ b | 9.7 x 10⁷ ± 2.0 x 10³ a | 5.1 x 10⁶ ± 1.3 x 10³ bc | -94.7 | -100 |
| TCCH5 | 2.03 x 10⁸ ± 2.0 x 10³ a | 8.5 x 10⁷ ± 2.3 x 10³ a | 4.9 x 10⁶ ± 7.1 x 10³ bc | -94.2 | -100 |
| TCCH7 | 2.04 x 10⁸ ± 1.6 x 10³ a | 8.4 x 10⁷ ± 3.0 x 10³ a | 3.7 x 10⁶ ± 1.4 x 10³ c | -95.5 | -100 |
| TCCH8 | 2.01 x 10⁸ ± 1.3 x 10³ ab | 6.4 x 10⁷ ± 1.4 x 10³ a | 1.5 x 10⁷ ± 3.3 x 10³ a | -76.2 | -100 |
| TCCH9 | 1.96 x 10⁸ ± 5.6 x 10³ c | 9.0 x 10⁷ ± 3.6 x 10³ a | 7.5 x 10⁶ ± 1.2 x 10³ ab | -91.6 | -100 |
Means (± standard deviation) followed by different letters in a column are statistically different according to Tukey’s test (P < 0.05). SDA + YE = Sabouraud Dextrose Agar + 0.1 % yeast extract.
Conidial production on rice
Conidial production on rice varied significantly among isolates (p < 0.0004) (Table 4). The strains that showed the highest conidial production were TCCH5, TCCH7, and TCCH8, with 2.03 × 10⁸, 2.04 × 10⁸, and 2.01 × 10⁸ conidia∙g⁻¹ of rice, respectively. The isolate with the lowest production was TCCH9, with 1.96 × 10⁸ conidia∙g⁻¹. According to García-Ortiz et al. (2015), conidial production is a critical factor for the success of biological control using entomopathogenic fungi. The strains that exhibited the highest conidial production on rice did not correspond with those that showed the highest production on SDA + YE medium. As noted by Cova et al. (2009), rice is the most commonly used substrate for the mass production of entomopathogenic fungi at the commercial level.
Pathogenic characterization
Figure 4 shows that all M. brunneum isolates exhibited pathogenicity toward A. tripterus, with significant differences (P < 0.0053) in effectiveness. The isolates that caused the highest mortality rates were TCCH5, TCCH7, and TCCH8, with no significant differences between them. However, the highest mortality rates were observed in TCCH5 and TCCH8, with values of 96.4 % and 89.7 %, respectively, at 8 days post-inoculation. The isolate that caused the lowest mortality was TCCH2, with 72.2 %. These results are consistent with those of Resquín-Romero et al. (2020), who evaluated M. brunneum isolates on the stink bug Euschistus heros Fabricius (Hemiptera: Pentatomidae); these authors reported mortality rates ranging from 83.3 to 100 % in nymphs and adults at 8 days post-inoculation by immersion. Other M. brunneum isolates have also caused mortality in insect species such as Bactrocera oleae Rossi (Diptera: Tephritidae) (60 % mortality at 9 days) and Agriotes spp. (44.2 % mortality at 45 days) (Razinger et al., 2018; Yousef et al., 2013). Additionally, M. anisopliae isolates have shown 100 % effectiveness on the stink bugs Nezara viridula L. in a period of 8 to 10 days (Abdel-Raheem et al., 2011) and Dichelops melacanthus Dallas (Hemiptera: Pentatomidae) (Groth et al., 2017).
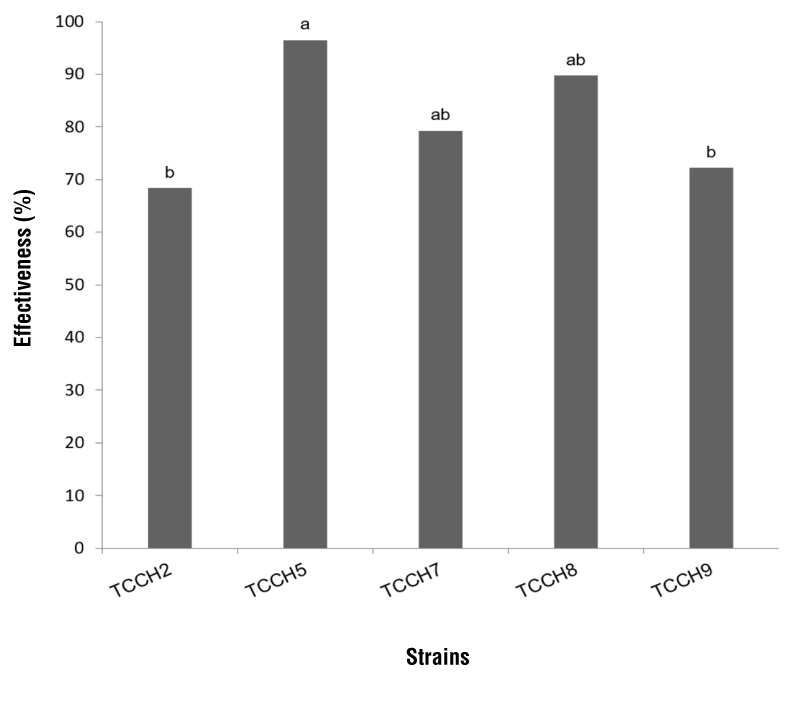
According to Barrios et al. (2016), the selection of the most promising isolates is essential for obtaining entomopathogenic fungi suitable for development as biopesticides capable of exerting effective regulation of the target pest. To this end, various characteristics of the isolates have been considered, including virulence, inoculum production, growth, sporulation, and tolerance to adverse environmental conditions (García-Ortiz et al., 2015). Based on these criteria, the most promising isolates in this study were TCCH5 and TCCH8. Other studies have also demonstrated the effectiveness of native entomopathogenic fungal isolates against pest species (Clifton et al., 2019; Hernández-Trejo et al., 2019).
Conclusions
The species Metarhizium brunneum was identified as an agent associated with the mortality of the black stink bug Antiteuchus tripterus in cacao plantations in Tabasco, Mexico. The M. brunneum strains exhibited variability in mycelial growth, germination time, conidial production, and pathogenicity. All fungal isolates showed pathogenicity against A. tripterus under laboratory conditions, with effectiveness ranging from 72 to 96 %. The native isolates of M. brunneum showed a favorable temperature range of 25 to 30 °C. Based on the evaluated characteristics, isolates TCCH5 and TCCH8 are the most promising as biological control agents for A. tripterus. This study reports, for the first time, the pathogenicity of M. brunneum against A. tripterus, contributing to the understanding of entomopathogenic fungal diversity. Field studies are necessary to evaluate the performance of the selected isolates under natural conditions.